


The three factors of light, progress and teamwork are illustrated in our group logo: Light (colored rays), which originates from several pieces that come together as a sphere symbolizing a team, illuminates the path of progress (arrow).
Motivation
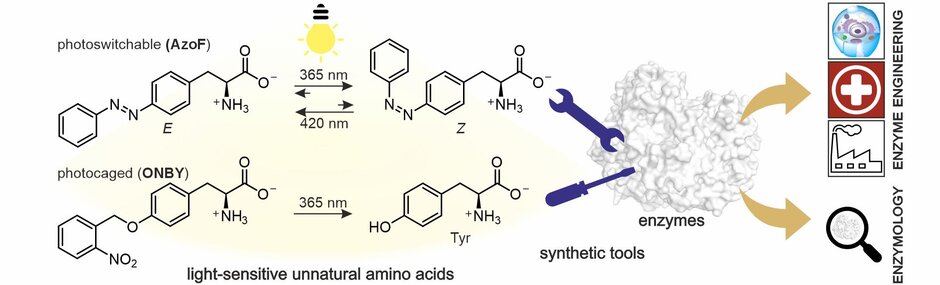
Enzymes are the most fascinating molecular machines in cells. It is thus of utmost interest to decipher their functional mechanism in the field of enzymology and to tune their function for various applications in the field of enzyme engineering. To achieve the powerful spatiotemporal control of enzyme activity, we work with lightsensitive unnatural amino acids (UAAs), which are incorporated via the expansion of the genetic code by amber suppression. Our overarching research goal is to leverage these UAAs as synthetic tools for fundamental enzymology studies and application-based enzyme engineering (Figure 1). Importantly, we call the lightsensitive enzymes generated in this process photoxenases.
Research focuses


Enzymology
In enzymology, particularly photocaged UAAs (Figure 1, bottom) are extremely valuable for extended mutagenesis studies. Their bulky sidechain allows to evoke different mutational effects than those of natural amino acids. More importantly, they convert to natural amino acids upon irradiation so that the regeneration of wild-type-like enzymes can be investigated with temporal resolution, e.g., by spectrometric methods or in X-ray experiments.
Tryptophan Synthase
Tryptophan synthase (TS) is a prominent multi-enzyme complex, which channels a substrate/product between two subunits. Notably, the two reactions at the active sites of the TrpA and TrpB subunits (Figure 2) are strictly regulated via allostery. Channeling of the substrate/product indole and allosteric regulation are both tightly connected to the so-called COMM domain.
Recently, we have shown that both indole channeling as well as allosteric events can be blocked by the incorporation of the photocaged UAA ONBY (Figure 1) [11], and restored upon light-induced conversion to tyrosine. With this synthetic tool in hand, we now aim to further investigate the interplay between conformational changes, indole transport and catalysis in a timely resolved manner.

Photoxenase Engineering
The spatiotemporal control of enzymes is of increasing interest for various applications. Photocontrol with photocaged UAAs (Figure 1, bottom) is straightforward and useful for diverse applications, particularly the control of cellular processes or the visualization thereof via controlled imaging [21] in cell research. However, the irreversible light-induced "decaging" of these UAAs also limits their scope. Photoswitchable UAAs (psUAAs; Figure 1, top) instead offer the reversible regulation of enzyme activity by a light-induced switch between two isomers, which is particularly important for applications in red and white biotechnology.
Notably, the design of reversible photocontrol has largely remained challenging. We strategically advance the engineering of reversible photocontrol by developing, understanding and initially applying switchable photoxenases.


Development
We consistently work on the following challenges, for which we have already achieved some initial successes [19, 20, 22, 23]:
- What kind of interactions between the psUAA and the enzyme are beneficial for efficient photocontrol?
- Can we boost the photocontrol efficiency and if so by which strategies?
- What are the requirements on the enzyme target and the position of psUAA incorporation?
- Can we develop engineering strategies that are applicable universally or at least to a subgroup of enzymes with the same property?
- Is it possible to control catalysis directly?
Understanding
In order to further develop a method, it is essential to understand the underlying mechanisms. Our recent findings [19, 23] showed that reversible photocontrol is based on a change in the conformational landscape of the enzyme. We are particularly interested in the following aspects:
- Is the thermodynamic stability of the enzyme states and thus the equilibrium between them or the states themselves and thus their productivity/activity changed by light?
- How is incomplete reversibility explained and how can it be improved?
- Do the light-induced changes affect only one step in the catalytic mechanism or several?
- How does signal transmission from the psUAA to the active site work?


Application
In terms of reversible photocontrol, we focus particularly on biotechnological applications in biotherapy and industrial biocatalysis.
Glutaminases are important therapeutic enzymes in the field of antibiotic and chemotherapy research. We work primarily with the allosteric imidazole glycerol phosphate synthase [10, 12, 20, 23] and asparaginase-glutaminase type II (Figure 6) [19], which is already established as a chemotherapeutic agent.
The pursuit of sustainability in industry is leading to the increasingly frequent use of enzymes as biocatalysts. Photocontrol is attractive for overcoming challenges such as different stability half-lives and side reactions in multi-enzyme cascades. Our goal is the photocontrol of various relevant enzyme systems for biocatalysis.
Genetic Code Expansion
For the efficient incorporation of our light sensitive UAAs we employ the amber stop codon suppression technology, Which is outlined in Figure 7. An orthogonal aminoacyl-tRNA synthetase (O-aaRS) is redesigned for binding the UAA and coupling it to an orthogonal tRNA (O-tRNA). At the ribosome the anticodon of the O-tRNA binds to a reprogrammed stop codon allowing the nascent protein chain to react with the UAA. The result of this reprogrammed protein synthesis is a protein bearing an UAA at a specified position.
The generation of photoxenases, and xenoptoteins in general, is largely limited by the high expense of (ps)UAAs due to low synthesis yields and low incorporation efficiencies. In our most recent projects we aim to tackle these limitations by various approaches.
